

Make someone’s day: Gift a subscription to your friends and family!
Twelve thousand years ago, the earth was covered with wild abundance. Countless species of plants, animals, and birds flourished across every continent. Yet among this biological wealth, only a tiny fraction would ever be domesticated, and those few species would become the foundation of civilization itself.
Wheat, barley, rice, lentils, goats, sheep, pigs, and cattle: all descended from wild ancestors that happened to live in certain fortunate regions. Those regions became the birthplaces of horticultural societies, and through them, the first steps toward the modern world.
Material progress, the key theme of this Substack and my book series, means the sustained improvement in the material standard of living of a large group of people over a long period of time. It is not simply the accumulation of wealth or the appearance of luxury; it is the transformation of ordinary life: better food, shelter, health, and security for the masses.
Human history shows that material progress has not been evenly distributed across time or geography. Some societies advanced rapidly, others remained trapped in subsistence for millennia. The reasons for this unevenness begin not with culture, intelligence, or moral character, but with geography and the raw materials that nature provided and the constraints it imposed.
To go through a transformation of the material standard of living of the masses, a society must first go through a number of preceding transitions that are only possible in certain geographies. It was only quite recently with the invention of the industrial technologies by Britain that societies were able to escape the geographical traps.
This essay pays homage to two thinkers who illuminated these foundations of civilization. The first is Nikolai Vavilov, the Russian botanist who mapped the world’s centers of plant domestication and revealed the biological diversity upon which agriculture depended. The second is Jared Diamond, whose book Guns, Germs, and Steel reawakened public understanding of how geography shaped the preconditions of history.
Vavilov’s and Diamond’s ideas help explain how the natural endowment of each region shaped the earliest transitions from wild landscapes to settled societies, and how those first transitions laid the groundwork for everything that followed: agriculture, trade, cities, industry, and the global progress that defines our age.
First, I would like to be very clear. Geography is not a cause of human material progress. Geography is a constraint on material progress: a set of boundaries and opportunities that societies must work within.
Some geographies made it possible to advance toward greater complexity; others made it nearly impossible until technological revolutions broke the limits. The Fertile Crescent, northern China, and parts of Mesoamerica possessed an abundance of wild plants and animals that could be domesticated. In contrast, regions such as sub-Saharan Africa, Australia, and North America lacked species suitable for early domestication, forcing their inhabitants to remain hunter-gatherers or simple horticulturalists until foreign crops, animals, and industrial technologies arrived.
It was Nikolai Vavilov and Jared Diamond who helped us understand those geographical constraints. In this article, I would like to present their ideas and expand them to achieve a better understanding of the material preconditions of progress.
Thesis: The global distribution of wild ancestors of plants and animals enabled the evolution of Horticultural societies. Horticultural societies were necessary steps in the evolution of more complex societies, such as Agrarian, Commercial, and Industrial societies. It was in the latter two society types that material progress for the masses evolved.

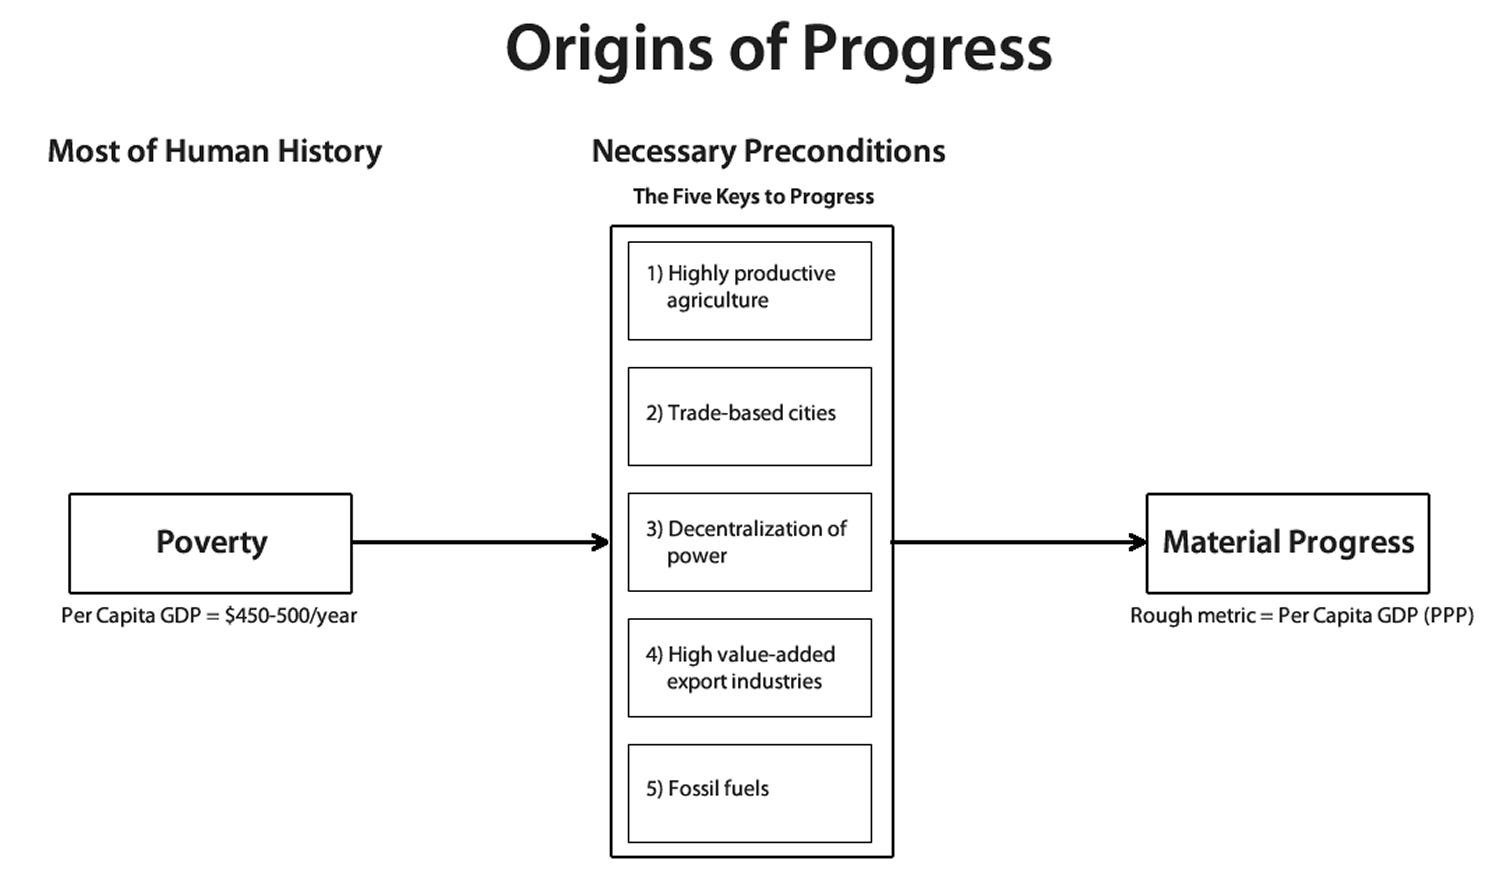
Or to put it another way, highly productive agriculture is the First of the Five Keys to Progress. The First Key was also the by far the hardest of the Five Keys to Progress to achieve because of the geographical constraints described in this article. The vast majority of human societies simply did not live in regions where it was possible, and the very low material standard of living of their people was the result.
If you enjoy this article, you should read my From Poverty to Progress book series.
Vavilov’s Vision and Diamond’s Synthesis
The story of how humanity began to master its natural environment begins not with kings or conquerors, but with a quiet Russian scientist walking through fields of grain. In the early twentieth century, Nikolai Ivanovich Vavilov undertook one of the most ambitious scientific missions of his age: to map the world’s original centers of cultivated plants.
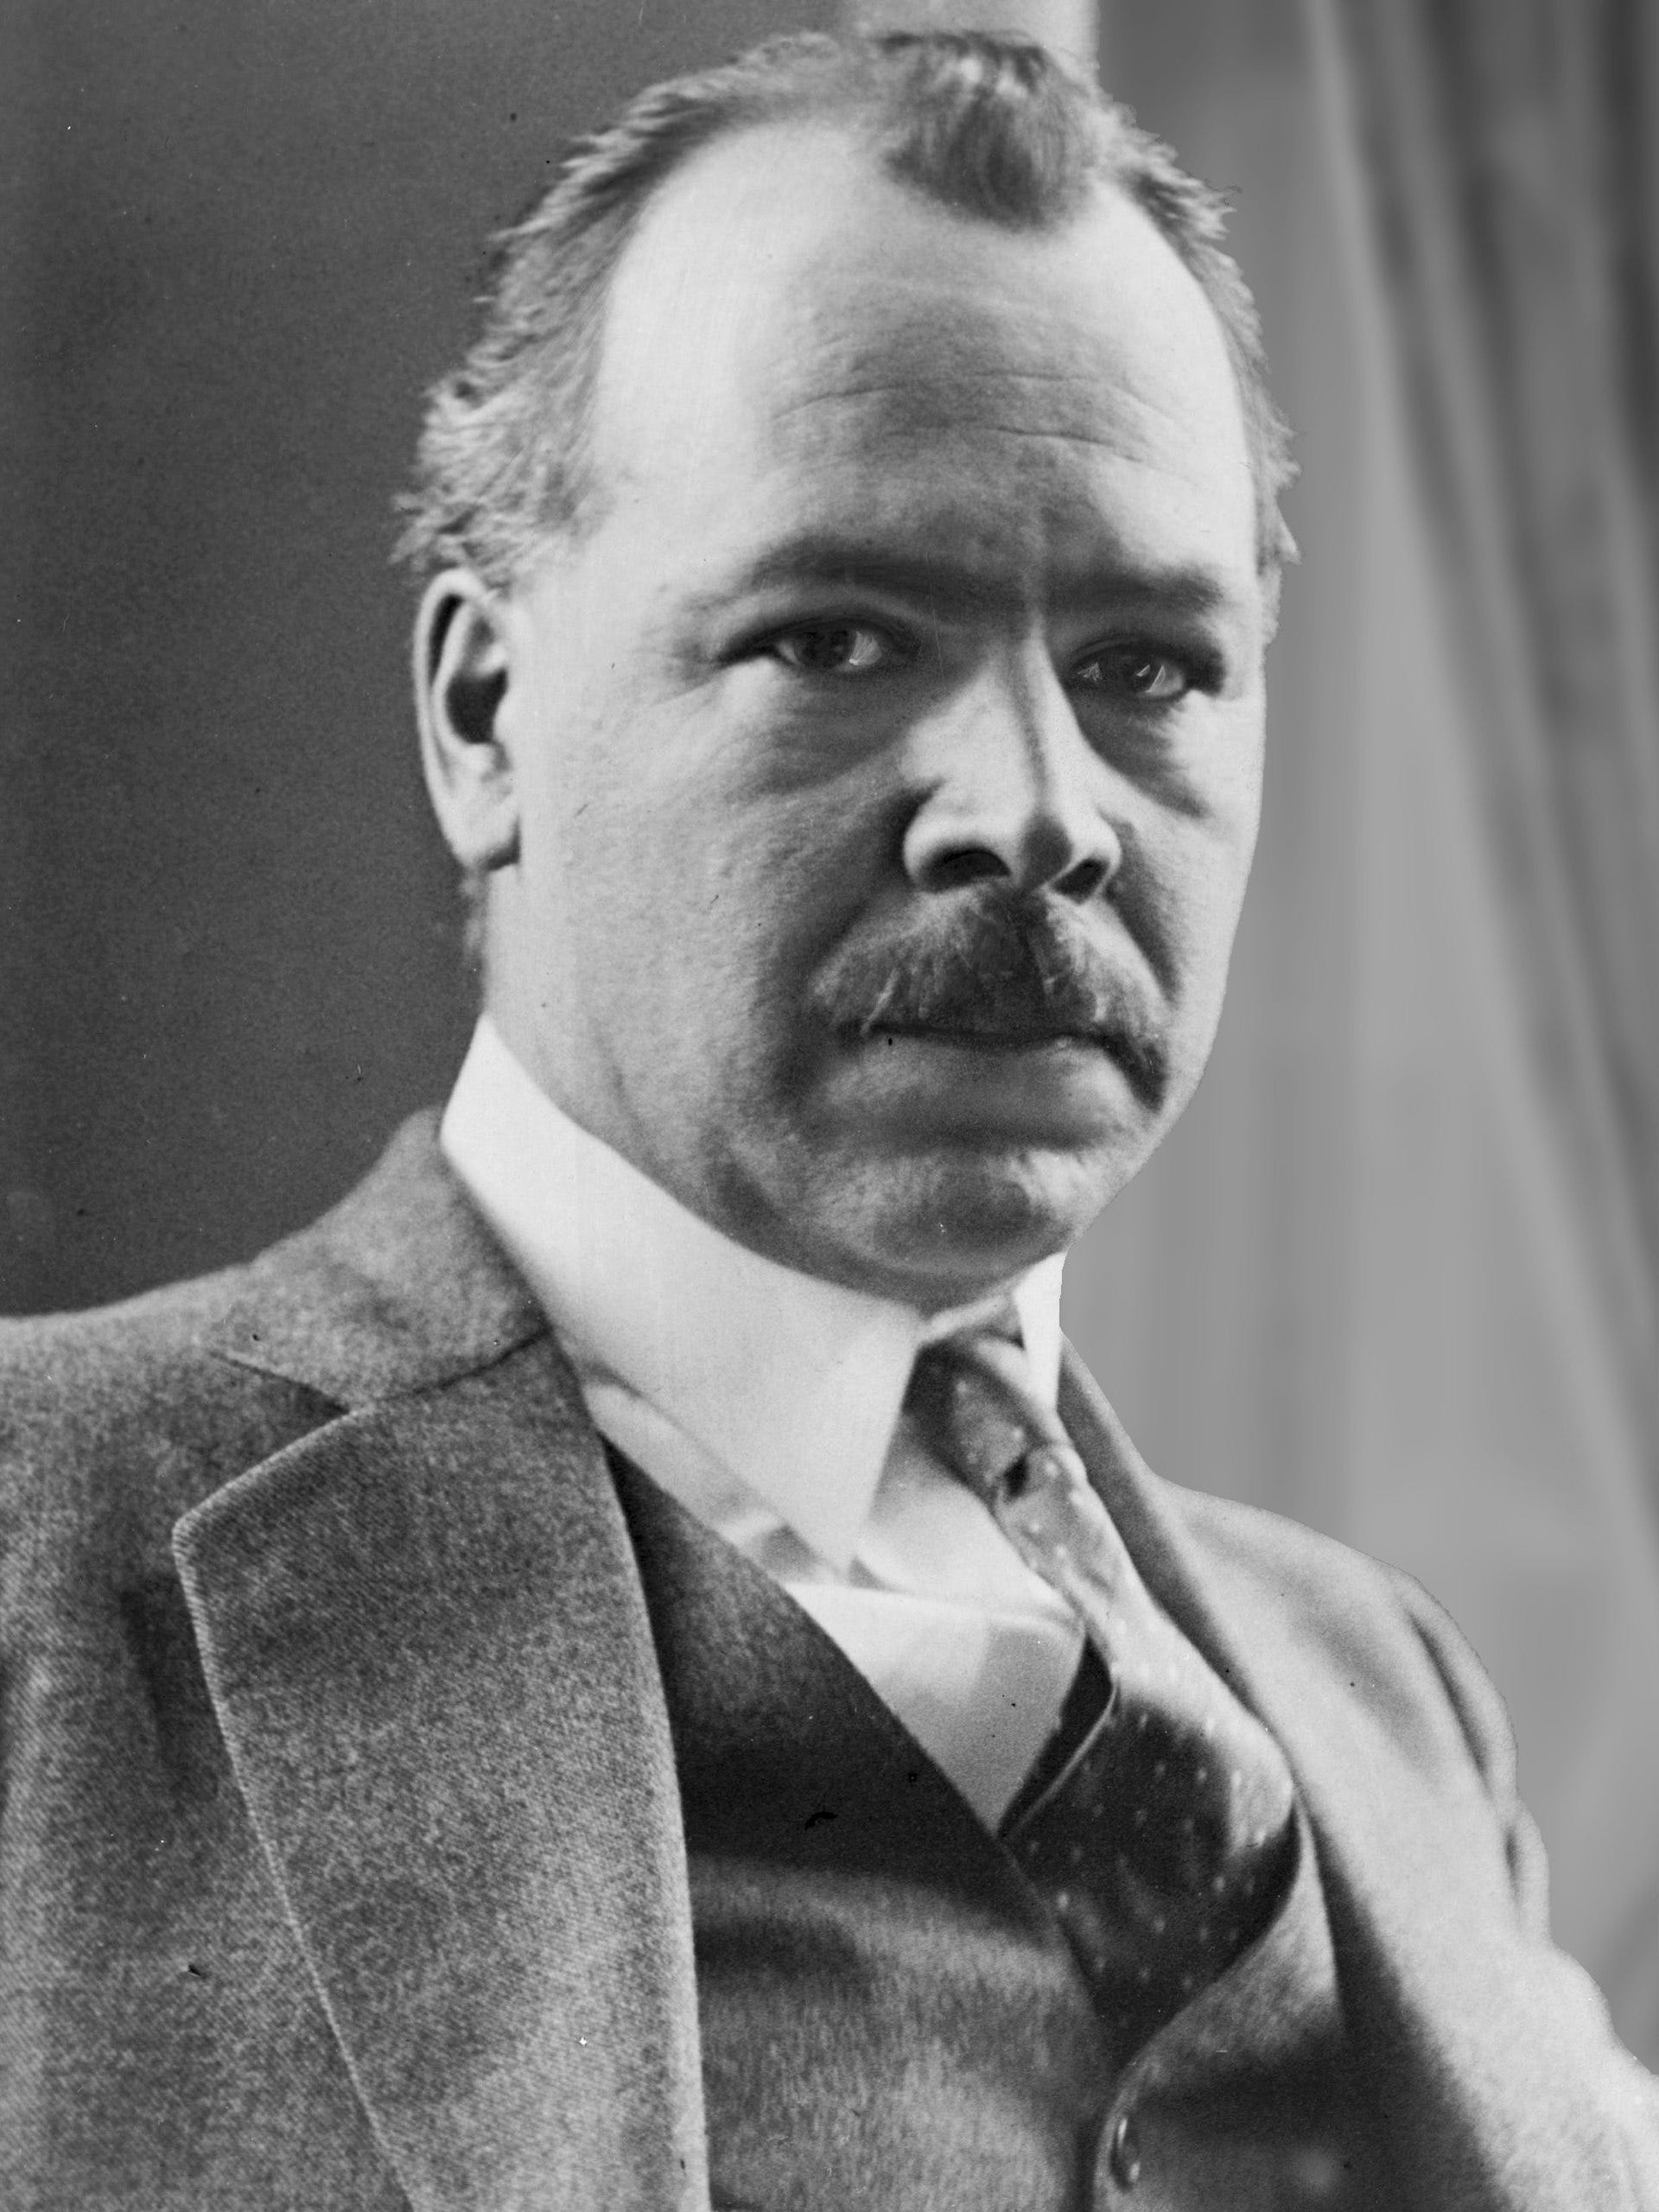
Traveling from the mountains of Afghanistan to the highlands of Ethiopia, from Central America to the Chinese interior, he collected hundreds of thousands of seeds and documented the local varieties that sustained human life. What Vavilov discovered reshaped biology and geography alike: domesticated crops had not arisen everywhere but only in a few exceptional places where nature’s wild abundance made cultivation possible.
Vavilov’s insight was deceptively simple. If one mapped the diversity of a crop’s wild relatives, one could find its center of origin, the region where it had first been domesticated. By this logic, wheat and barley trace back to the Fertile Crescent, rice to East Asia, maize to Mesoamerica, and potatoes to the Andes. These were the regions where nature had placed the right combination of wild species, climate, and soil to permit early cultivation. Humanity’s future was, in a sense, built on the luck of this biological draw. Vavilov understood that the range of wild ancestors set the outer limits of what early societies could achieve.
Geography did not dictate outcomes. Geography defined possibilities. Possibilities that technological innovations in subsistence technologies could exploit given enough time for experimentation.
This was the first great scientific articulation of geography as constraint rather than cause. The people of the Fertile Crescent did not invent agriculture because they were more intelligent or industrious than the peoples of Australia or sub-Saharan Africa; they did so because their environment offered the materials from which agriculture could be made. In other regions, the absence of suitable wild species closed off the path entirely.
Vavilov never used the language of progress or civilization, but his maps implied a profound truth: the evolution of complex societies depended on the geography of wild biodiversity.
Vavilov’s achievements were vast, but his life ended tragically. He became one of the first victims of Soviet political science. His insistence on genetics and empirical evidence brought him into conflict with Trofim Lysenko, whose pseudoscientific theories pleased Stalin’s regime. His theory was later termed Lysenkoism and rejection of it was seen as an ideological rejection of the Communist project.
Tragically, Vavilov was arrested, starved, and eventually died in prison in 1943. Vasilov’s seed collections left neglected in the cold.
For decades, Vavilov’s name was suppressed in the East and forgotten in the West, and his ideas survived mainly in the archives of agricultural institutes. Today, few outside the scientific community remember him, yet much of modern botany, genetics, and food security rests on his foundations.
Half a century later, Jared Diamond would take up the same question from a new direction. In Guns, Germs, and Steel (1997), (summary here) Diamond asked why Eurasian civilizations had conquered the world while others remained technologically less advanced. His answer revived and expanded Vavilov’s central insight: geography and ecology, not innate human differences, shaped the broad pattern of world history.
Diamond argued that Eurasia’s wide range of domesticable plants and animals combined with its east–west orientation, which allowed easy diffusion of species gave the continent a decisive early advantage. Over millennia, these advantages compounded into dense populations, powerful states, and advanced technologies.
Where Vavilov catalogued the raw materials of domestication, Diamond explained their consequences. His synthesis linked biology, geography, and history into a coherent narrative of human development. Though some critics accused him of determinism, Diamond repeatedly emphasized that geography was not a cause of success but a framework of constraint. Diamond say geography as a set of ecological boundaries within which human societies either flourished or faltered. His book did not reduce culture to nature; it explained why some environments allowed cultural evolution to accelerate while others imposed ceilings that could not be broken until industrial technology arrived.
I read Diamond’s book when it was first published and loved it. It is exactly the kind of history book that I most enjoy: it is vast in scope while being clear in theory and impressive in its level of evidence presented. And though my thinking has moved far beyond Diamond’s theory, it is still one of my all-time favorite books.
Guns, Germs, and Steel transformed popular understanding of history. It shifted attention from moral or racial explanations to environmental and structural ones, and in doing so, it revitalized the study of how geography shapes the possibilities of progress.
Yet even Diamond’s achievement was incomplete. He captured the broad environmental foundations of early inequality but not the full range of geographical constraints that continued to shape societies long after agriculture. Some geographies limited the diffusion of trade, the concentration of skilled labor, or the ability to sustain complex institutions. My own theory treats all of these factors as essential to understanding how progress evolved.
I have written a number of articles on these other geographical constraints on the evolution of human societies that go far beyond what Vavilov and Diamond wrote:
Why Progress Started Where It Did (more on biomes)
More ways geography has constrained human progress (rivers, altitude, soil)
How progress spreads to neighboring societies (human geography)
Why are there such huge variations in income across the globe?
Still, both Vavilov and Diamond deserve enduring credit: they revealed that the first step toward civilization was not invention but adaptation to the possibilities nature allowed.
The Biology of Domesticated Plants: Nature’s Genetic Gatekeepers
When early humans first began to cultivate plants, they did not yet know they were performing one of the most profound biological experiments in history. Each seed they gathered and replanted was a data point in a vast evolutionary trial testing which species could adapt to human hands. Over centuries, this unconscious experiment reshaped both plants and people.
Humanity became dependent on a narrow set of species that evolved under cultivation, and those species in turn became dependent on humanity for survival. The partnership was not designed; it was discovered. And the conditions for that discovery were not evenly distributed. Nature’s genetic architecture created zones of opportunity where cultivation could take root, and vast regions where it could not.
Modern genetics has revealed just how rare the right biological traits for domestication truly are. In People, Plants and Genes: The Story of Crops and Humanity, (summary here) biologist Denis Murphy describes the domestication of plants as a form of coevolution, a biological dialogue between human selection and plant adaptation.
The process was not the product of deliberate design but the unintended consequence of everyday behavior. Hunter-gatherers who repeatedly harvested the most productive or accessible wild stands of grain unknowingly biased the next generation of plants. Proto-horticultural societies that re-sowed the best seeds near their camps or favored certain plots for convenience were performing selective breeding long before they understood the concept. Over generations, such unconscious preferences reshaped entire species.
Domestication, in other words, began as an accident of success.
People returned to the richest patches of wild grain year after year because those areas yielded the most food, not because they intended to transform nature. By cutting seed heads before they shattered, they preserved the genetic variants that retained seeds on the stalk longer. By threshing and replanting near settlements, they favored plants that germinated easily in disturbed soil.
What looked like habit or convenience became, at the population level, a powerful evolutionary filter. The result was that the wild plants most useful to humans evolved to depend on human activity for reproduction, while humans evolved socially and culturally around their new plant partners.
The evolutionary logic of crop domestication
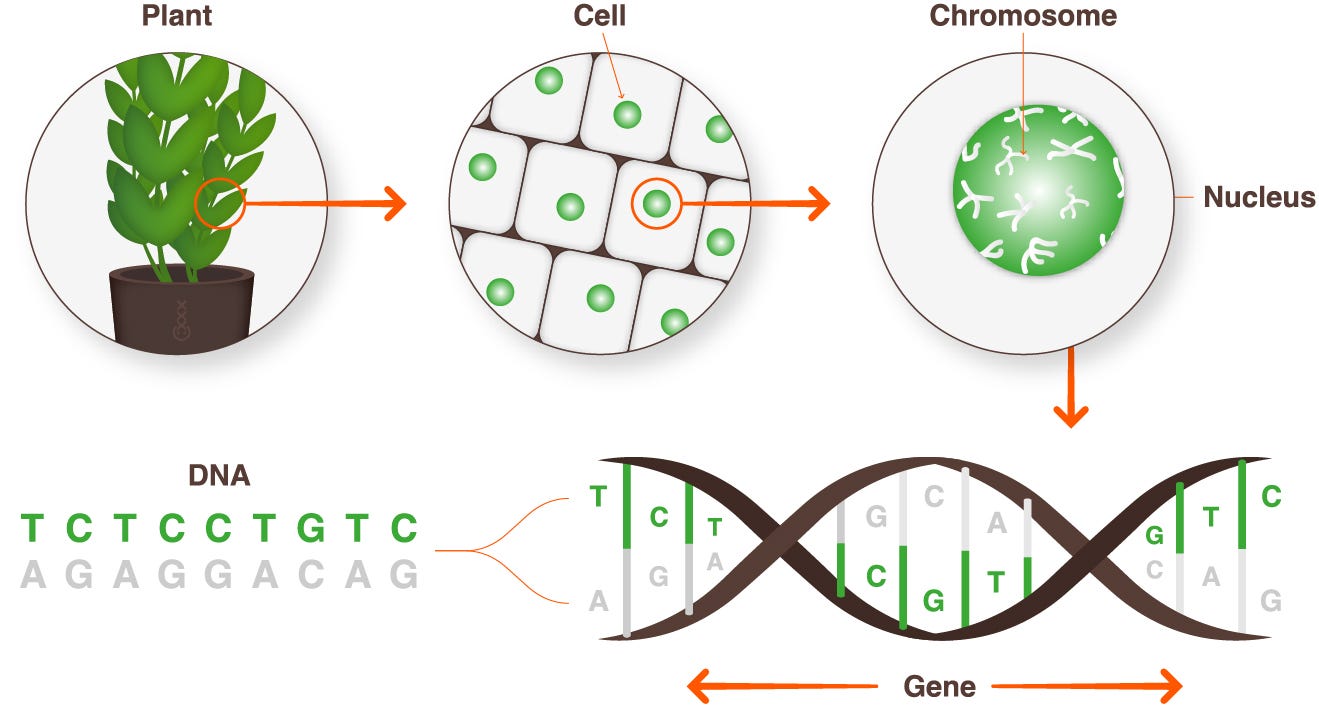
The first farmers did not consciously select for specific genes, but their habits of gathering, storing, and replanting created strong selective pressures. Seeds that stayed attached to their stalks until harvest, that sprouted quickly after sowing, or that produced larger grains were favored. Over time, these repeated preferences transformed wild populations into domestic varieties. The most important of these changes involved the non-shattering gene, which prevents seeds from dispersing before harvest, and the loss of dormancy, which synchronizes germination. Together they turned wild grasses into crops. What looks like simple replanting was in fact a massive evolutionary filter operating over thousands of years.
Certain biological properties made some species more responsive to this process than others. Annual life cycles allowed rapid genetic turnover, speeding selection. Self-pollination stabilized useful mutations. Polyploidy (the possession of multiple chromosome sets) produced genetic flexibility and hybrid vigor, as in wheat, cotton, and potatoes. Many of the great domesticates are polyploids, because their genetic redundancy gave them extraordinary adaptability. These traits are not evenly distributed in nature; they are evolutionary accidents. Geography therefore determined not only where suitable wild species existed, but also where their genetic architectures allowed domestication to succeed
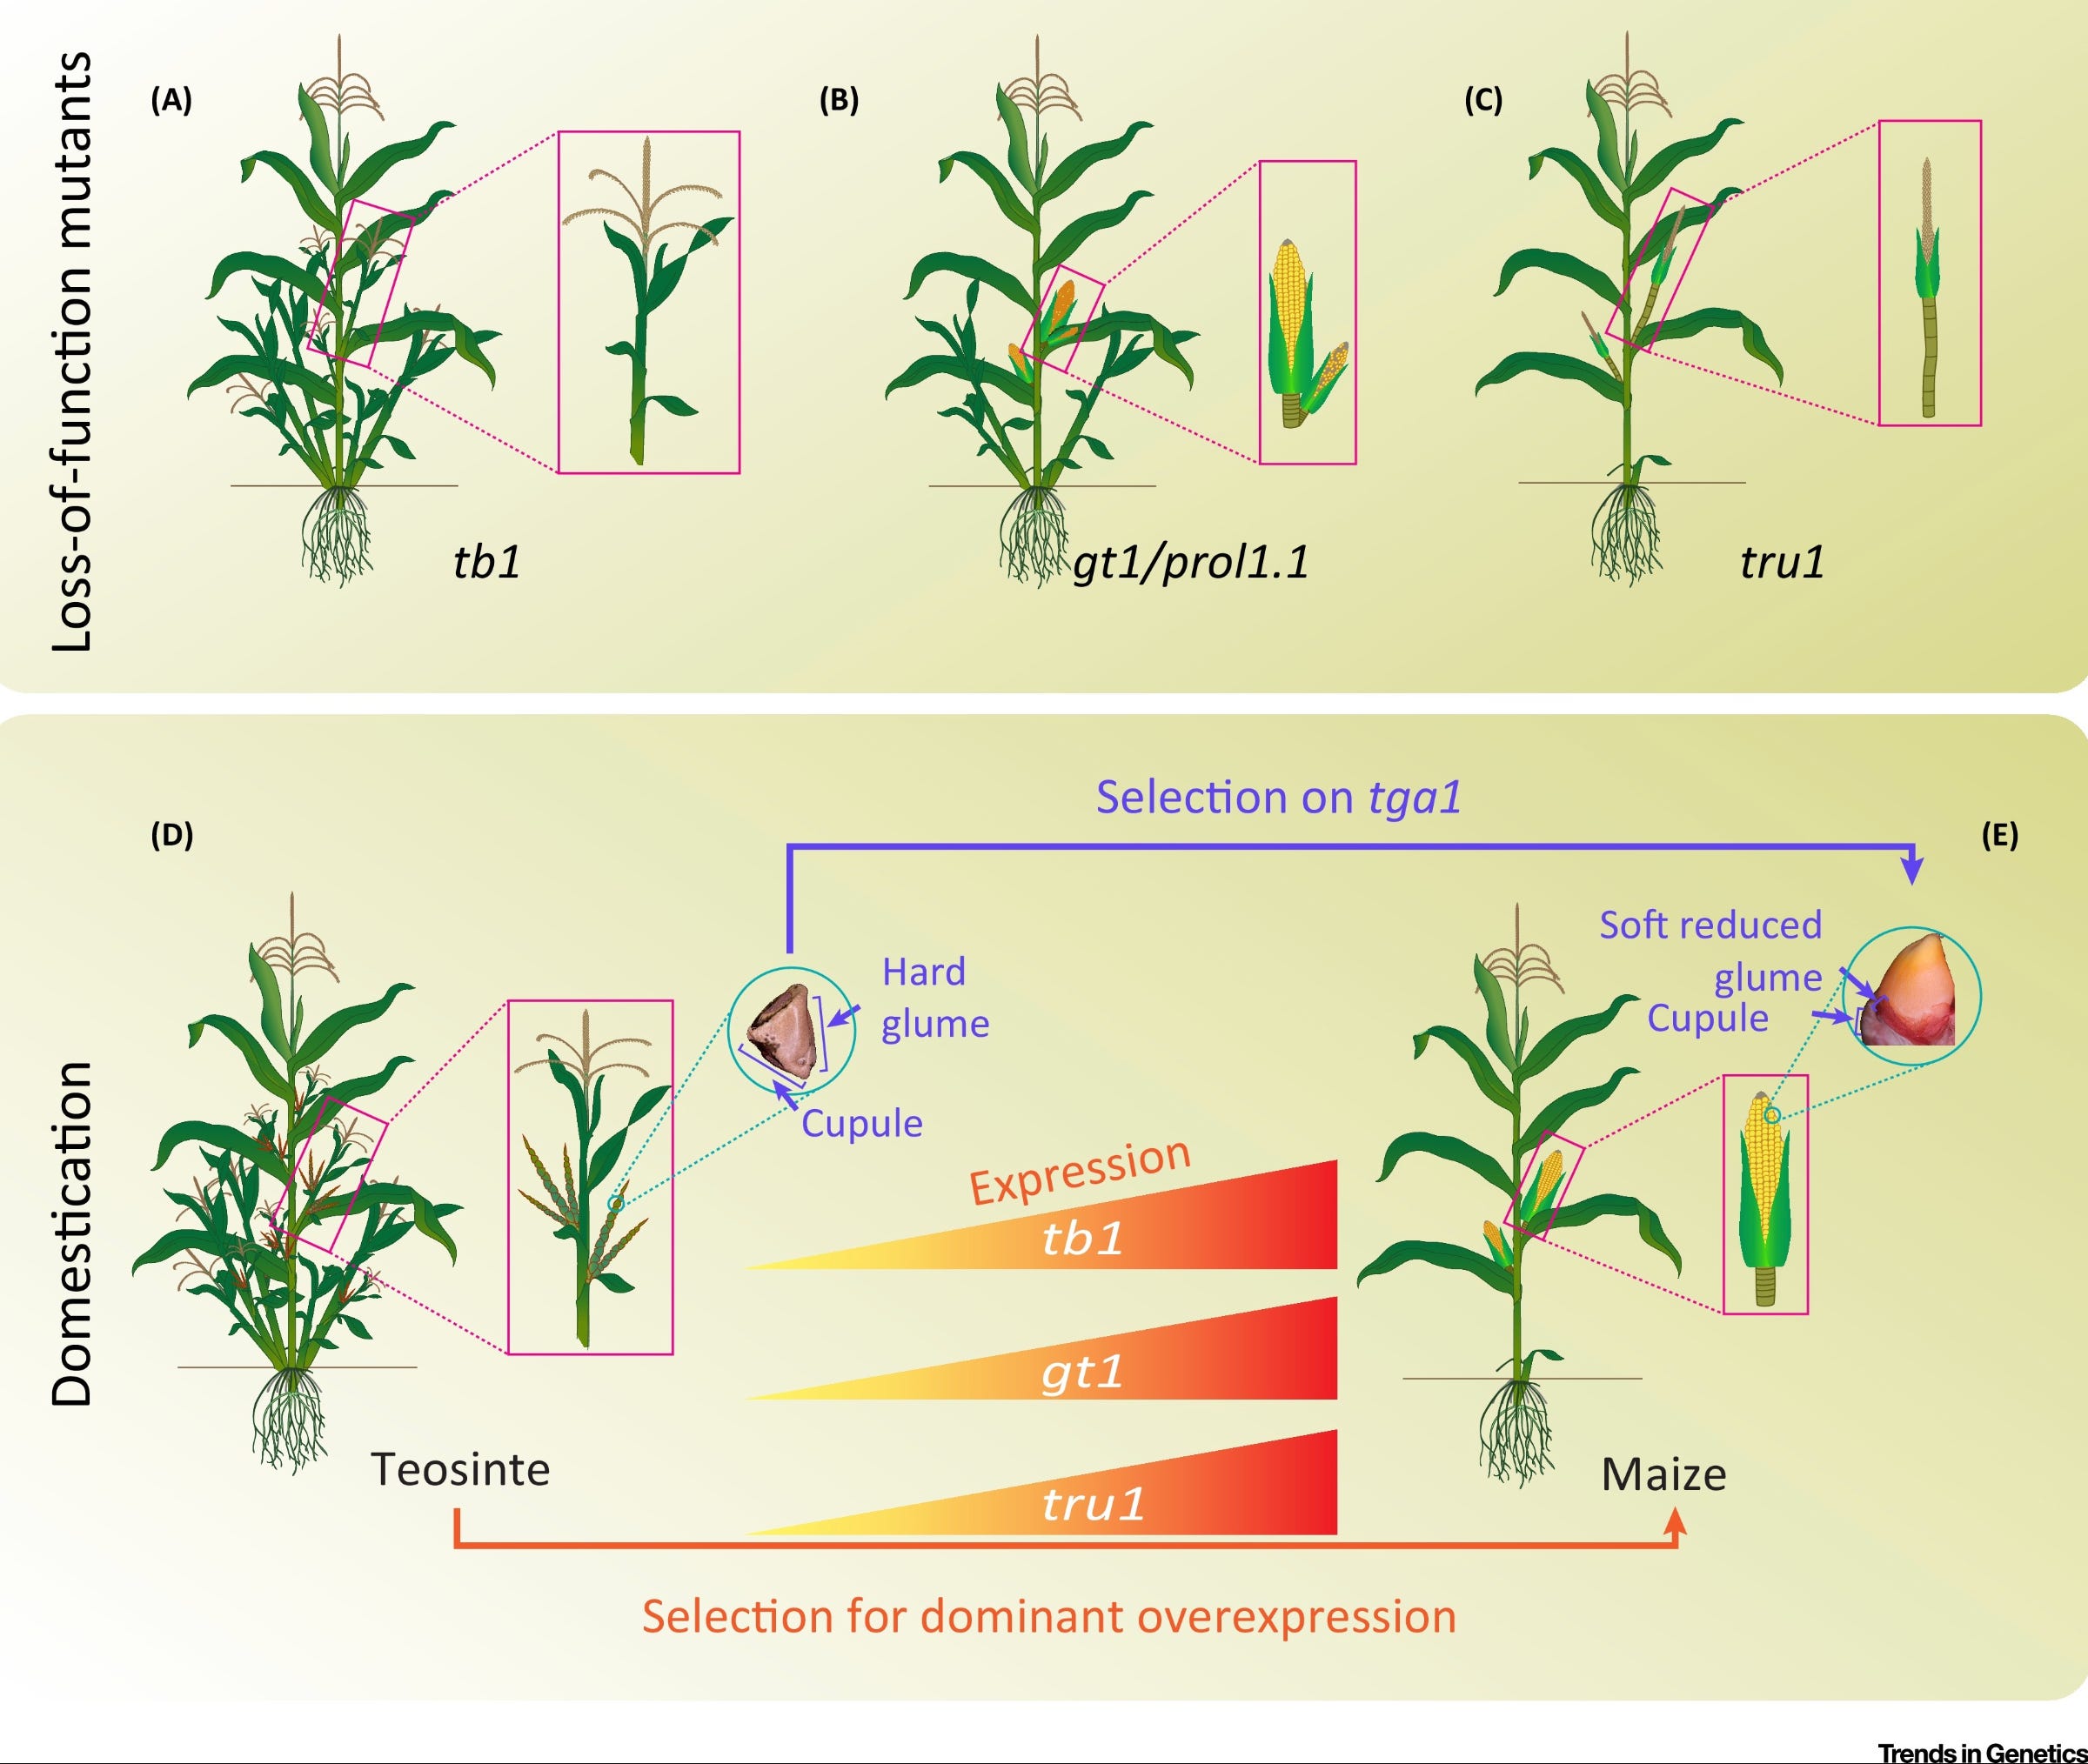
The biological characteristics of domesticable plants
Across species, domesticated crops share a recognizable suite of traits that made them unusually malleable under human selection. The most important are:
Annual or short life cycles that allow rapid generational turnover and quick reinforcement of desired traits.
High seed yield per plant, concentrating energy into edible structures rather than vegetative growth.
Non-shattering seed heads, which make harvesting efficient.
Loss of seed dormancy, producing uniform germination when sown.
Self-fertility or flexible pollination systems, allowing stable inheritance of advantageous mutations.
Phenotypic plasticity, or the ability to adapt to different soils and climates.
Tolerance of crowding and cultivation, which permits intensive planting.
At the genetic level, these features have a common theme: they are governed by relatively simple mutations with large effects. It is this genetic property of the wild ancestors of staple crops that made domestication probable even by accident.
A single change in a transcription factor can suppress seed shattering or control flowering time. Many domestication traits arise from mutations in regulatory genes, genes that act as master switches controlling cascades of other traits. This architecture made certain plants extraordinarily responsive to human selection.
With just a few generations of replanting, wild grasses could be transformed into cereals. The simplicity of the underlying genetics explains why domestication occurred independently in multiple regions: once the right raw material existed, the path was open.
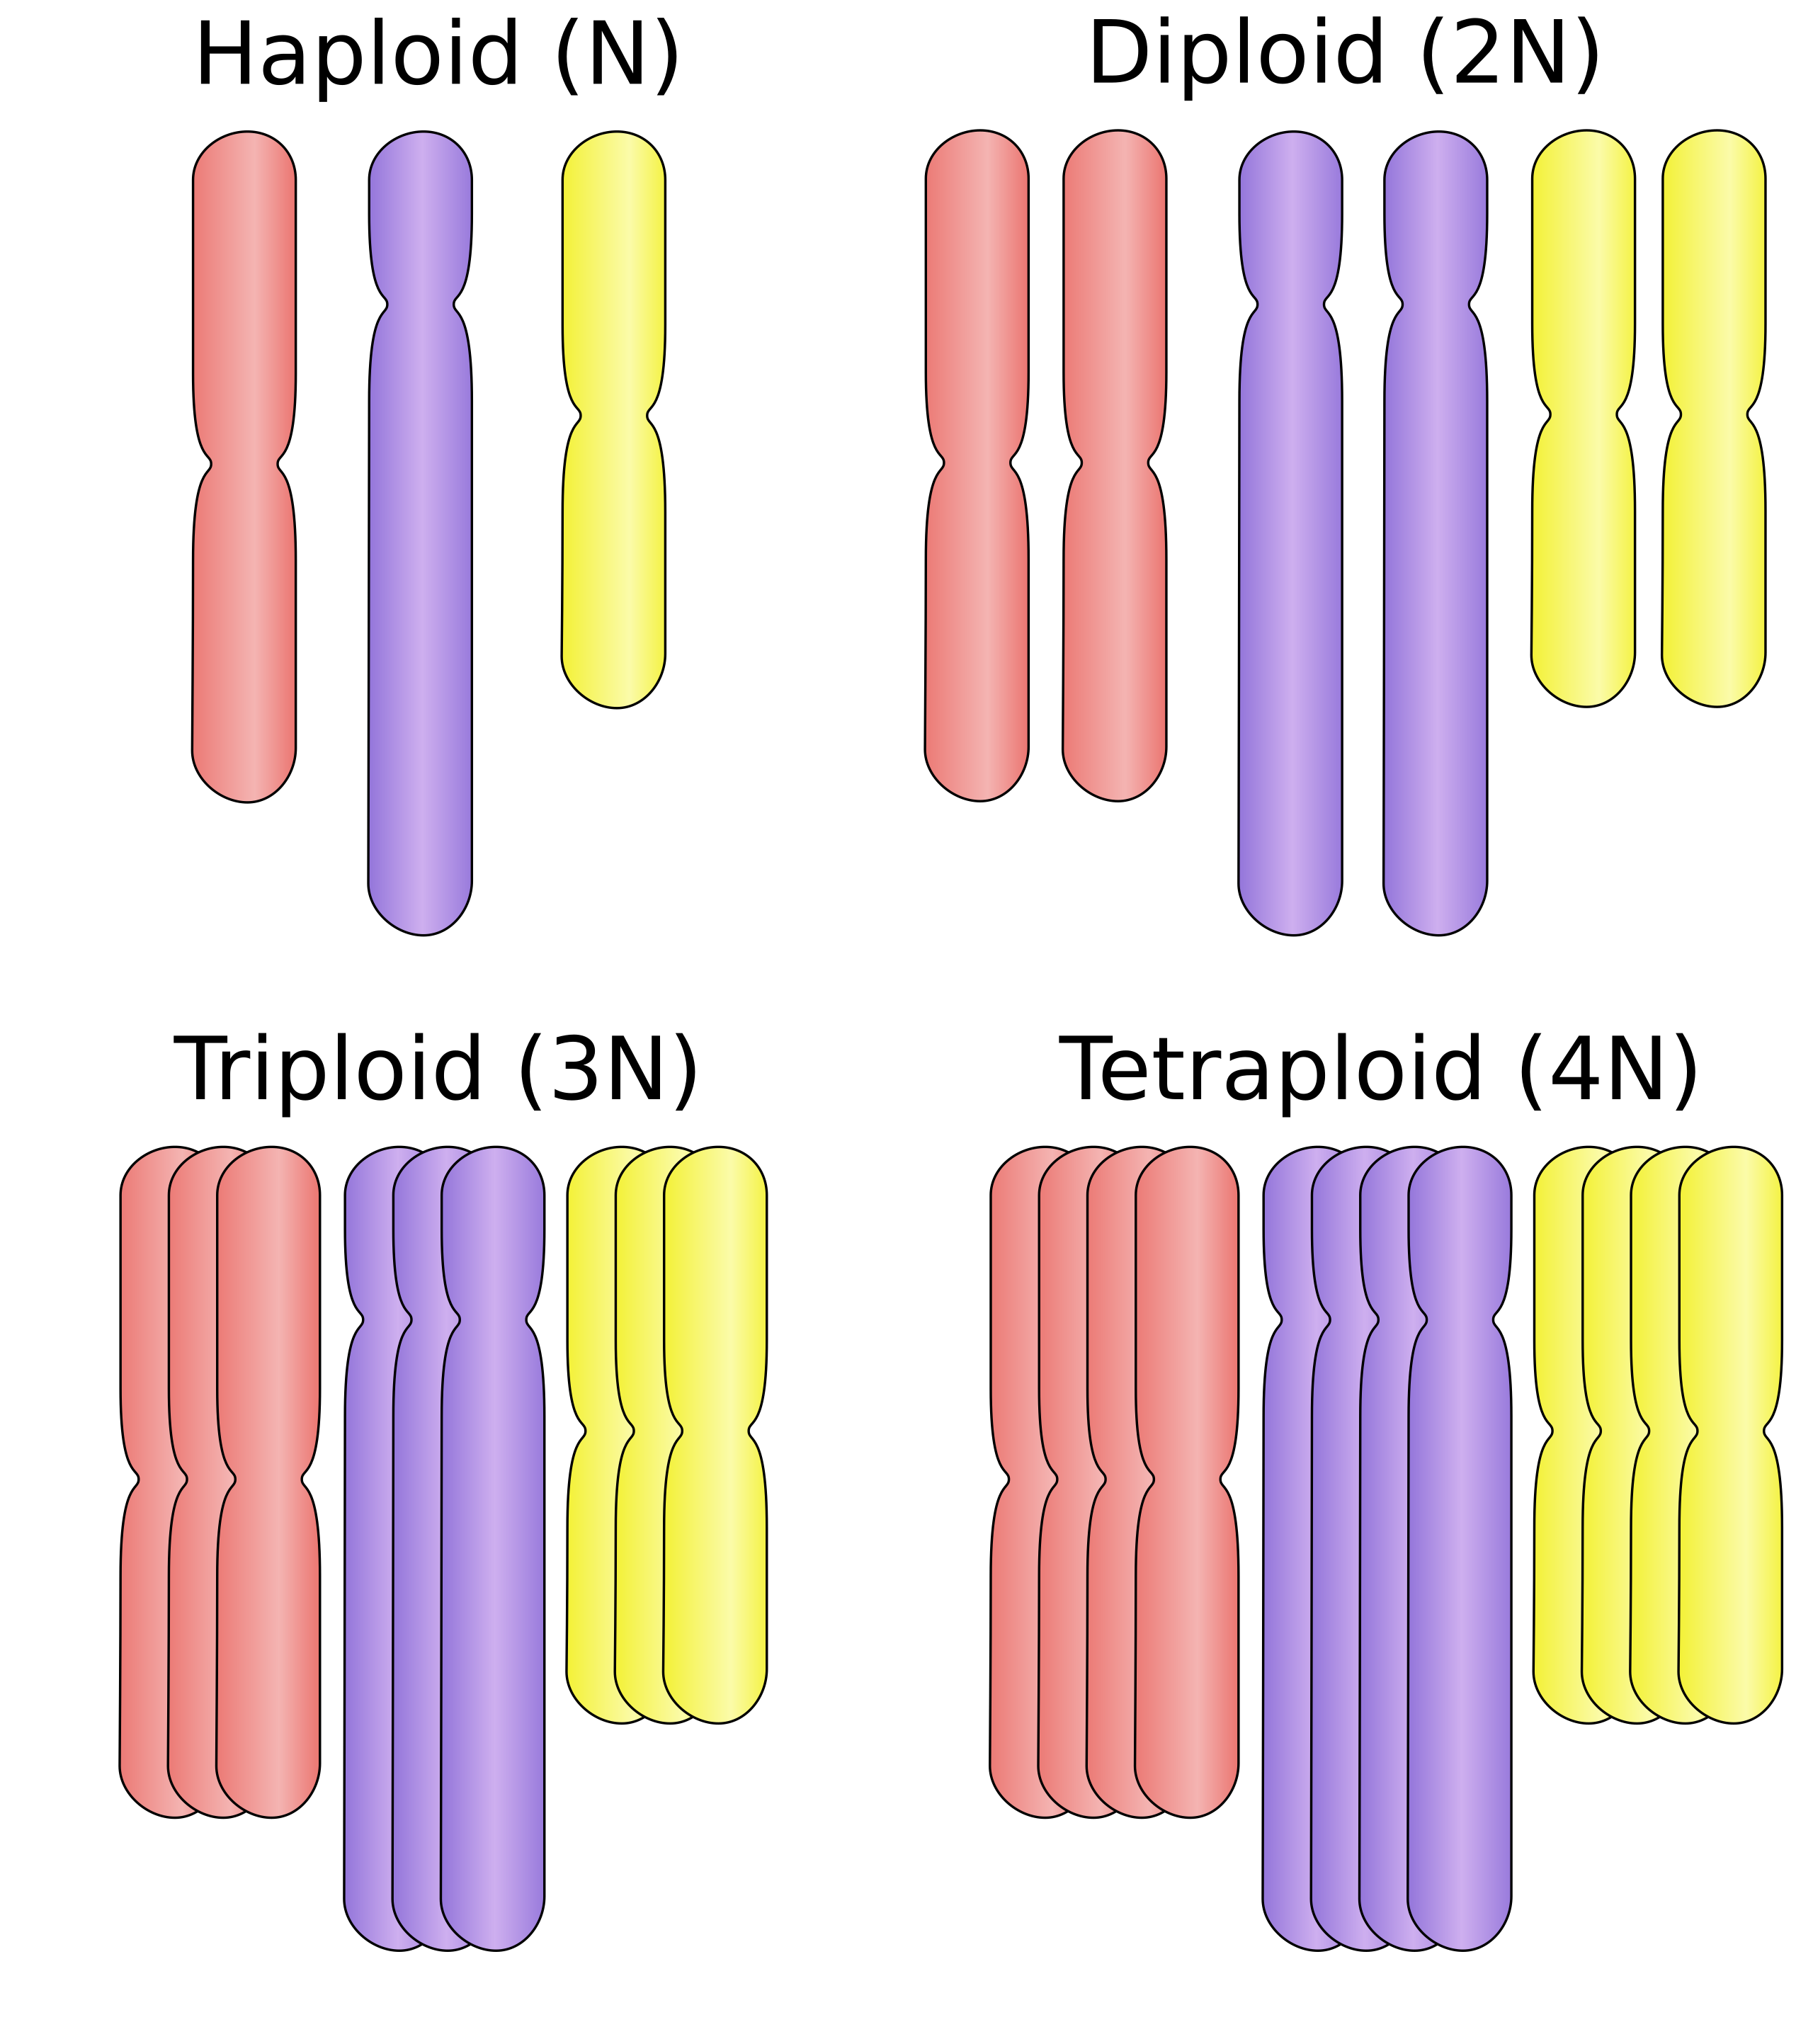
Polyploidy added another layer of malleability. Polyploidy is a condition in which the cells of an organism have more than two paired sets of (homologous) chromosomes.
Extra chromosome sets create redundancy, allowing one copy of a gene to mutate without lethal consequences. This freedom accelerates the evolution of useful traits such as larger seeds, disease resistance, and adaptability to new climates. Many of humanity’s staple crops, such as wheat, oats, cotton, potatoes, are polyploids, and their genetic flexibility made them resilient under cultivation and migration. In effect, polyploidy turned certain species into open systems ready for continuous improvement, while others remained genetically brittle.
Nature’s uneven distribution of opportunity
Murphy’s analysis deepens Vavilov’s insight: the world’s crop centers were not arbitrary cultural zones but biological ones.
The Fertile Crescent, China, Mesoamerica, Andean South America, and sub-Saharan Africa each contained clusters of species with genetic traits conducive to domestication. In contrast, large portions of Australia, Siberia, and North America lacked plants with these traits entirely. It was not intelligence or ingenuity that separated early horticultural societies from foragers; it was the presence or absence of wild species whose genomes could be reshaped by human hands.
The result was an uneven global map of potential progress.
In the Fertile Crescent, wild wheat and barley already possessed large seeds, brittle husks, and high yields. Only a minimal selection was needed to make them productive crops. In East Asia, rice and millet offered similar opportunities. In the Americas, maize required thousands of years of human selection to transform from a weedy grass into a staple grain, delaying agricultural intensification.
Other regions had nothing comparable. Even the most innovative peoples could not domesticate what nature had not prepared. Geography, again, acted as a constraint, not a cause, by defining which biological opportunities existed to be discovered.
The coevolutionary feedback loop
Once domestication began, the process accelerated through feedback. Cultivated plants became dependent on human activity for survival, while humans became dependent on cultivation for food.
This feedback created a new ecological niche that supported larger populations and more permanent settlements. The transition to horticulture was not simply a cultural change; it was a biological alliance between humans and certain plant species. Each harvest reinforced the selection pressures that made crops more productive, less hardy, and more reliant on human care. Humans, in turn, evolved culturally and socially to manage these delicate dependents developing calendars, storage methods, and eventually writing and trade.
This coevolution between people and plants marks one of the great turning points in the history of life. For billions of years, evolution had been governed by natural selection alone. With the rise of cultivation, artificial selection joined it as a new evolutionary force. Yet artificial selection could act only where natural variation made it possible. Thus, the biological properties of wild ancestors, encoded in their genomes long before humans, appeared became the hidden foundation of civilization.
The limits of biological inheritance
By shaping early food systems, the biology of domesticated plants defined what kinds of societies could arise. Horticultural societies built around grains could produce surpluses, while those dependent on tubers or fruits remained limited in scale. Cereal grains, such as wheat, barley, rice, millet, maize, offered a unique combination of high calorie density, storability, and portability. These characteristics enabled taxation, trade, and specialization: the first rudiments of complex society.
In this sense, Murphy’s genetic explanation complements Diamond’s geographical one: certain environments were hospitable to progress because they contained species with the right genetic plasticity to respond to human cultivation. Other environments were not.
The biological foundations of early agriculture reveal the dual nature of geography as both opportunity and constraint. The Fertile Crescent was not destined for greatness; it was endowed with plants whose genomes happened to unlock the path to horticulture. Australia was not destined for delay; it was limited by the absence of such species.
Only with the rise of industrial technologies, such as synthetic fertilizer, mechanized transport, and global trade, did humanity begin to escape these biological boundaries. But for ten thousand years, the map of human progress was written in the genetic possibilities of wild plants

The Biology of Domesticated Animals
If the cultivation of plants began as an accident of convenience, the domestication of animals began as an accident of proximity. Some species lived close enough to human camps to scavenge food, tolerate noise, and reproduce in the margins of human activity.
Over generations, these species adapted to the presence of people, and people learned to manage them. The first partnerships were not planned acts of mastery but emergent relationships formed by repeated contact. From this mutual adaptation arose one of the greatest biological alliances in history: a network of species that multiplied human strength, expanded food supplies, and transformed the ecological balance of the world.
The story of animal domestication parallels that of crops but operates on a different biological foundation. It was not only the physical traits of animals that mattered, but their behavioral genetics: their patterns of fear, aggression, and reproduction.
Where plants responded to selection through simple mutations in seed and growth genes, animals required complex alterations to their neuroendocrine systems. The crucial breakthrough was not learning how to breed animals for strength or milk but discovering, often unconsciously, which species were capable of forming stable hierarchies under human control. Only a few possessed this genetic potential, and they were clustered in certain regions of the world.
The evolutionary logic of animal domestication
Domestication began when particular wild species entered human ecological niches, not when humans decided to capture them. Wolves that scavenged near Paleolithic camps became less fearful, reproducing among themselves and eventually giving rise to dogs. Goats and sheep that tolerated herding pressure could be corralled and selectively bred.
In each case, the process began with self-selection: animals that were less aggressive toward humans enjoyed better access to food and protection. Humans, in turn, favored and protected the most docile individuals. This cycle of mutual accommodation gradually transformed both partners.
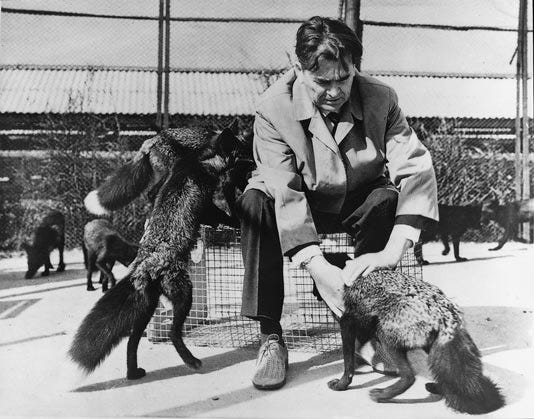
The most illuminating evidence comes from the Russian geneticist Dmitry Belyaev’s long experiment with silver foxes. By selecting only the tamest individuals for breeding, Belyaev produced animals that not only lost their fear of humans but also developed drooping ears, piebald coats, shorter snouts, and extended juvenile playfulness.
These physical and behavioral traits appeared together because they were genetically linked, a phenomenon now known as the domestication syndrome. Small genetic shifts in developmental and hormonal pathways produced large effects on both appearance and temperament. The same pattern recurs across species: the cow, the pig, the horse, the camel, and the dog all show similar clusters of traits. These were not random outcomes but the predictable results of selecting for reduced aggression and heightened sociability.
The biological characteristics of domesticable animals
Just as only certain plants possessed the right genetic architecture for cultivation, only a handful of wild animals possessed the behavioral and physiological foundation for domestication. The key characteristics were:
Dietary flexibility: Omnivorous or herbivorous species that could thrive on easily supplied food. Carnivores were too demanding or dangerous to feed.
Rapid growth and early sexual maturity: Species that reached reproductive age quickly and bred frequently could be managed sustainably.
Captive breeding tolerance: Willingness to mate in confinement, a rare trait among large wild mammals.
Predictable temperament and low flight response: Animals that did not panic in close quarters or attack humans could be herded.
Social hierarchy with a dominant leader: Pack or herd species accustomed to clear dominance structures could transfer that hierarchy to human handlers.
Group cohesion and follow-the-leader behavior: Essential for managing flocks and herds over long distances.
Low territoriality: Animals that could share space with others without conflict adapted best to domestic settings.
Each of these traits reflects underlying genetic and hormonal systems that make behavior flexible under selection. For example, the reduction of adrenal gland activity decreases fear and aggression; changes in neural-crest cell development alter pigmentation and ear shape while simultaneously influencing temperament. These shared pathways explain why the domestication syndrome appears across species. The genes that made an animal docile also made it physically juvenile, creating the familiar neoteny seen in dogs, pigs, and cattle.
In evolutionary terms, domestication is a process of permanent adolescence, a retention of juvenile plasticity into adulthood, maintained through human selection.
Geography as constraint and opportunity
The distribution of these biologically suitable species was strikingly uneven. Eurasia possessed most of the candidates:
goats,
sheep,
cattle,
pigs,
horses,
donkeys,
camels,
reindeer,
chickens.
The Americas had only llamas and alpacas in the Andes and turkeys in Mesoamerica. Sub-Saharan Africa’s zebras and antelopes were too skittish to breed in captivity; Australia had none. This pattern mirrors Vavilov’s crop centers: the Fertile Crescent and its surrounding zones held an extraordinary concentration of species already predisposed to domestication.
Geography did not cause domestication, but geography determined where the right genetic starting points existed.
In regions rich with domesticable animals, early horticultural and agrarian societies could multiply their productive energy. Oxen and horses plowed fields; camels carried goods across deserts; sheep provided wool; goats and cattle gave milk and meat. The result was a dramatic expansion of the human energy budget.
In regions without such species, humans remained the primary source of muscle power. Thus the geography of wild ancestors constrained not only the spread of agriculture but the pace at which societies could build surpluses, armies, and trade networks.
The coevolutionary feedback between humans and animals
Once domestication took hold, the relationship deepened into a feedback loop. Humans shaped animal behavior through selective breeding and training; animals reshaped human societies through their labor and products. Herding economies emerged on grasslands unsuited to crops, allowing humans to exploit vast new ecosystems. Milk, wool, and manure transformed diets and soil fertility. Animal traction increased the land area that one family could farm, magnifying agricultural output and accelerating population growth.
Over time, animals became extensions of human energy and identity: tools, companions, and sources of status. Yet the partnership remained rooted in biology: humans could domesticate only those species whose genes made them capable of cooperation. The rest, no matter how useful they might have seemed, remained forever wild. This was another form of natural constraint: the limits of animal temperament and development set the ceiling on how far early societies could mechanize their labor before the arrival of fossil fuels.
The legacy of biological partnership
The domestication of animals completed the transformation that began with plants. Together they created a self-reinforcing system in which energy, nutrition, and mobility increased hand in hand. Domesticated animals multiplied human reach, allowing larger communities, longer trade routes, and more specialized labor. They also changed the evolutionary trajectory of humans themselves, selecting for new skills, diseases, and immunities that distinguished agricultural peoples from their foraging ancestors.
The result was a world increasingly shaped by cooperation across species. The first steps toward civilization were not merely acts of human ingenuity but the consequence of biological compatibility, of finding in nature those species whose genes could align with human purpose. Geography determined where such partnerships were possible, and biology determined which species could enter them. Only much later, with industrial technology, could humans replace animal energy with mechanical power and finally transcend these ancient biological limits. But for most of history, progress depended on the simple fact that a few species, by the luck of evolution, were ready to become our allies.

The Biography of the Wild Ancestors
Behind every agricultural civilization stands a small group of plants and animals whose ancestors happened to inhabit the right landscapes at the right times. The pattern of their wild ranges reveals that the first great endowment of humanity was not cultural but geographic.
The Fertile Crescent, an arc stretching from the Levant through northern Mesopotamia into western Iran, contained an extraordinary concentration of species that met the biological criteria for domestication. In no other region did so many potential crops and herd animals coexist within a single climatic and ecological zone.
The major domesticated plants and their wild ranges
Wheat (emmer Triticum dicoccum, einkorn Triticum monococcum): Wild progenitors: T. urartu and Aegilops speltoides. Range: upland Levant, southeastern Turkey, and western Iran. Both species naturally hybridized in this region to produce emmer, which carried the non-shattering mutation crucial for harvesting.
Barley (Hordeum vulgare): Wild ancestor: Hordeum spontaneum. Range: Levant, Jordan Valley, and foothills of the Zagros Mountains. Early forms already showed semi-brittle rachis traits favorable to cultivation.
Lentil (Lens culinaris): Wild ancestor: Lens orientalis. Range: Fertile Crescent, especially northern Syria and southeastern Turkey.
Pea (Pisum sativum): Wild ancestor: Pisum humile. Range: Levant to western Iran.
Chickpea (Cicer arietinum): Wild ancestor: Cicer reticulatum. Range: southeastern Turkey.
Flax (Linum usitatissimum): Wild ancestor: Linum bienne. Range: eastern Mediterranean, Levant, and western Anatolia. Used for oil and fibers.
Olive (Olea europaea): Wild ancestor: Olea europaea sylvestris. Range: coastal Levant and Mediterranean basin; domesticated later in secondary diffusion.
Grape (Vitis vinifera): Wild ancestor: Vitis sylvestris. Range: Near East through the Caucasus to southern Europe; domesticated first in the Transcaucasus or Levant, then spread westward.
Date Palm (Phoenix dactylifera): Wild ancestor: Phoenix theophrasti and related species; native to Mesopotamia and the Arabian Gulf region. Provided fruit and sugar in arid zones.
These nine crops alone provided the basis for nearly every ancient Near Eastern diet. They shared critical traits: large seeds, annual life cycles, and compatibility with temperate rainfall patterns. Their wild ranges overlapped across a corridor only a few hundred kilometers wide, creating what Vavilov called a center of origin, a zone where the world’s first food system could evolve through selective gathering and replanting.
Outside the Fertile Crescent, similar clusters were far rarer.
In China’s Yellow River basin, the parallel system of millet (Setaria italica, Panicum miliaceum) and soybean (Glycine max) developed independently; along the Yangtze, rice (Oryza sativa, from wild Oryza rufipogon) became dominant. In Mesoamerica, maize (Zea mays from teosinte), beans, and squash formed another triad. In the Andes, potatoes (Solanum tuberosum) and quinoa (Chenopodium quinoa) were complemented by llamas.
Yet only the Fertile Crescent combined this many calorically dense crops within a compact ecological range and alongside large domesticable mammals.
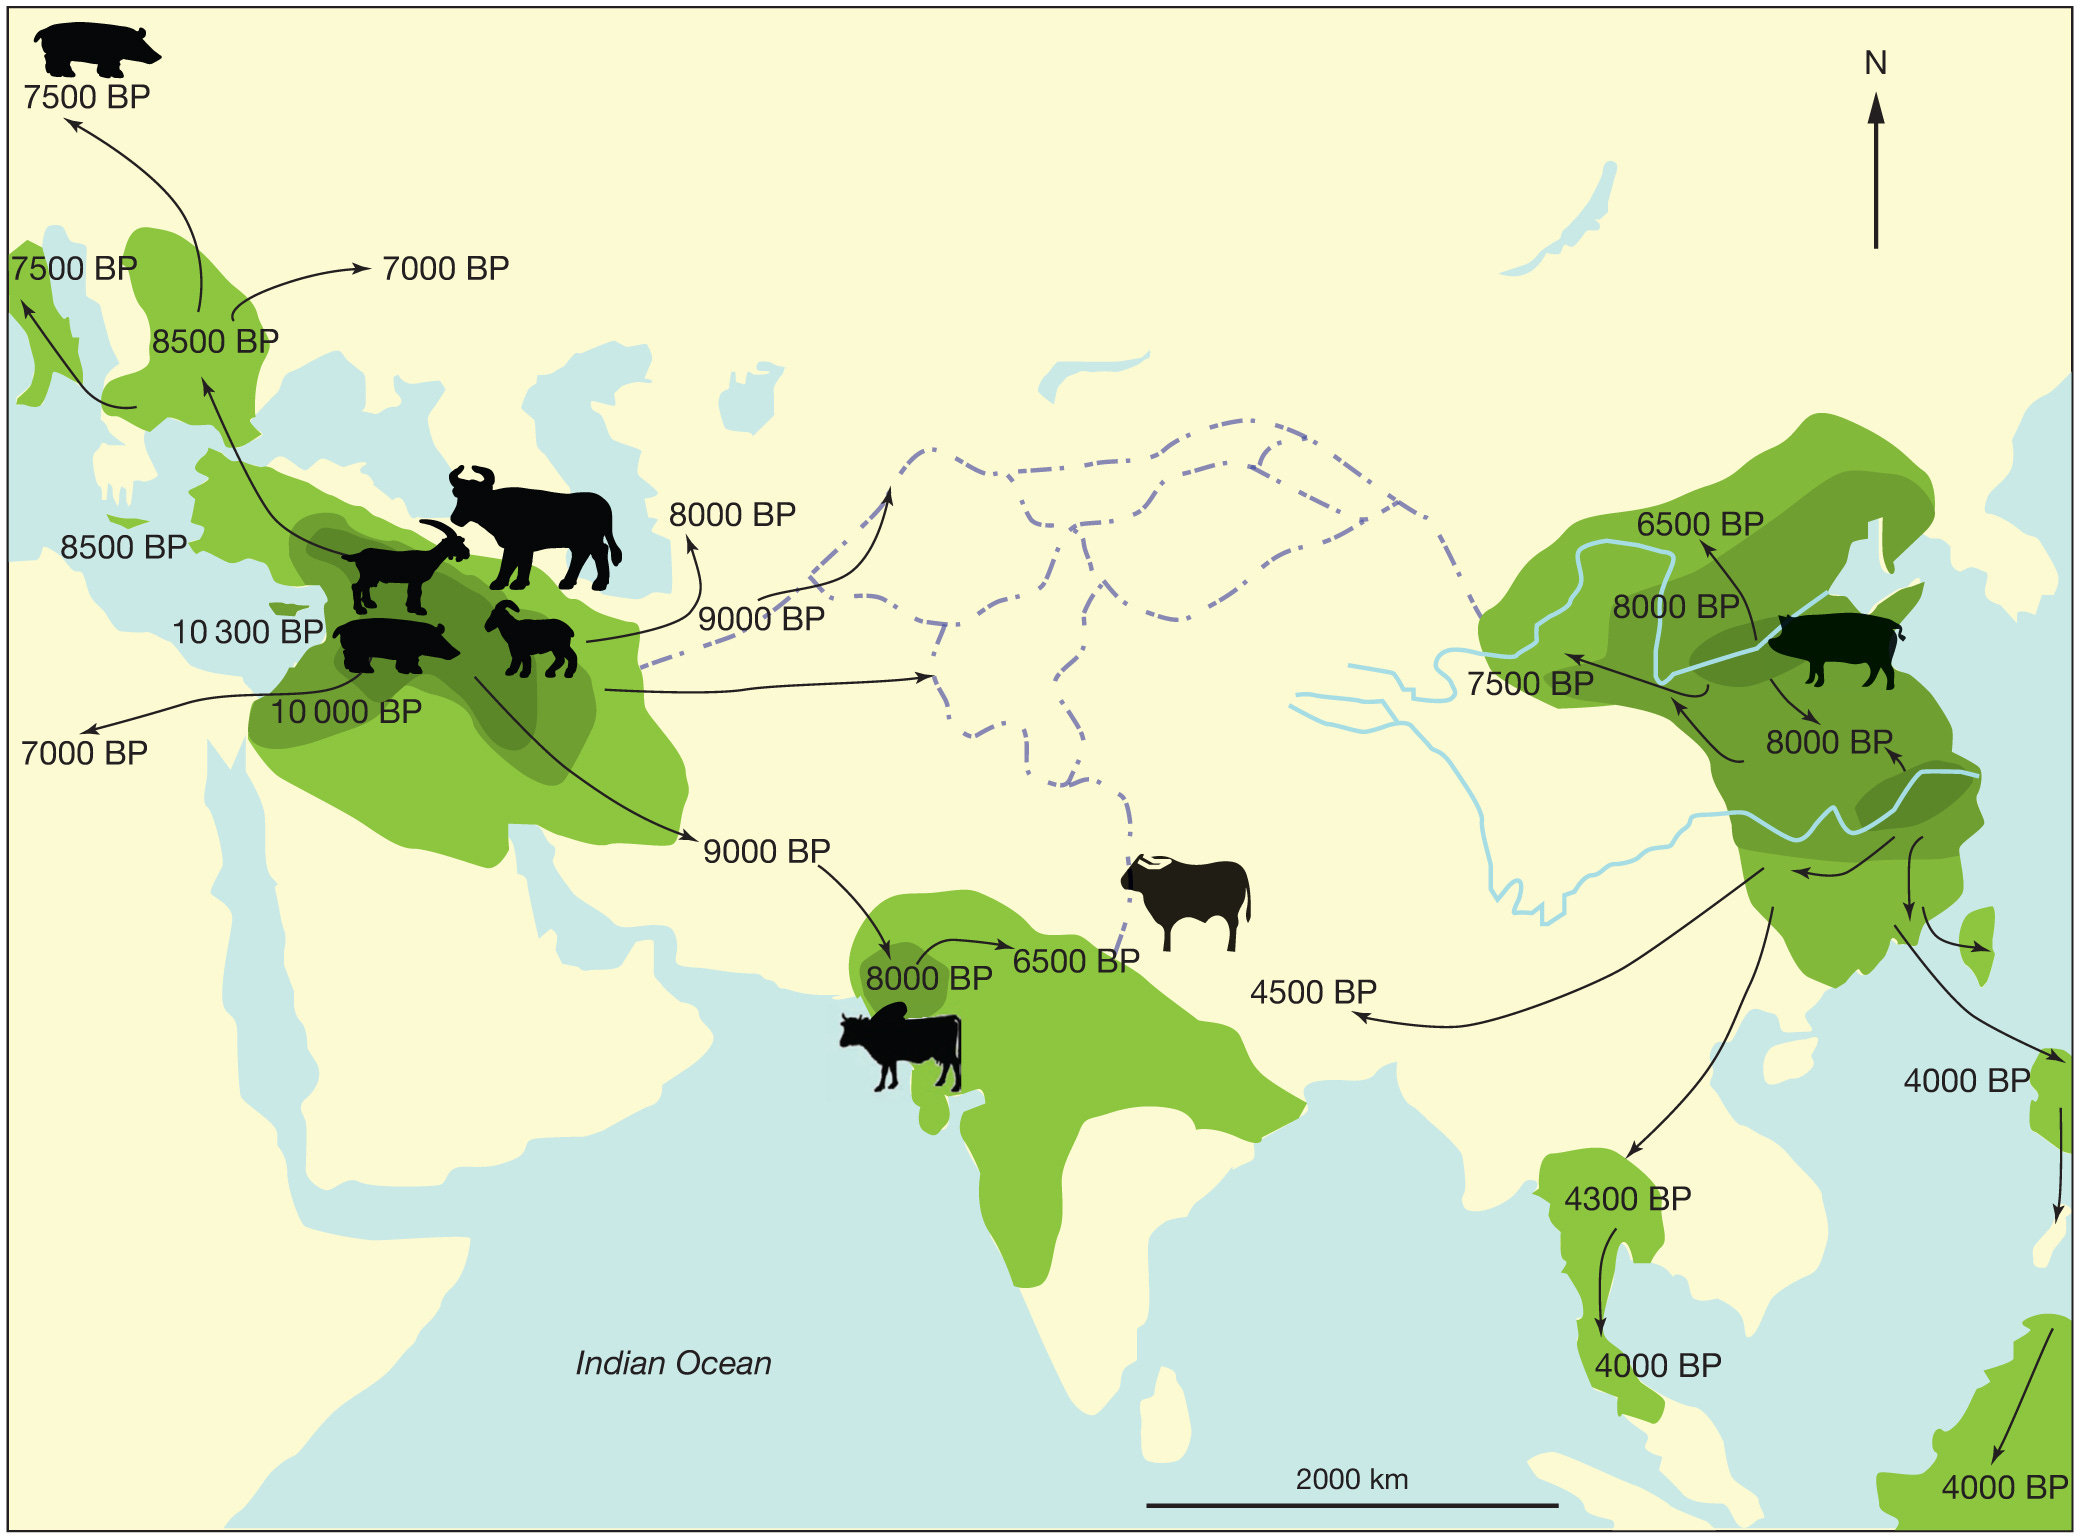
The major domesticated animals and their wild ranges
Goat (Capra hircus): Wild ancestor: Capra aegagrus. Range: Zagros Mountains of Iran and Turkey. First herded around 8500 BCE.
Sheep (Ovis aries): Wild ancestor: Ovis orientalis. Range: same highlands of the Fertile Crescent. Provided meat, wool, and milk.
Pig (Sus scrofa domesticus): Wild ancestor: Sus scrofa. Range: Anatolia through Europe and East Asia; independently domesticated multiple times.
Cattle (Bos taurus): Wild ancestor: Bos primigenius (aurochs). Range: temperate grasslands from the Balkans through the Levant to India; domesticated around 8000 BCE in the Fertile Crescent and again in the Indus Valley.
Dog (Canis lupus familiaris): Wild ancestor: Canis lupus (wolf). Range: northern Eurasia; likely self-domesticated near human camps before agriculture, but integrated early into agrarian economies.
Donkey (Equus asinus): Wild ancestor: Equus africanus (African wild ass). Range: Northeast Africa; domesticated in Egypt and diffused through the Near East.
Horse (Equus caballus): Wild ancestor: Equus ferus ferus. Range: Pontic–Caspian steppe north of the Black Sea; domesticated later (ca. 3500 BCE) but vital for transport and plow traction.
Camel (Camelus dromedarius, Camelus bactrianus): Wild ancestors: Arabian and Central Asian species; domesticated for desert and steppe trade routes.
Chicken (Gallus gallus domesticus): Wild ancestor: Gallus gallus (red junglefowl). Range: South and Southeast Asia; diffused westward in the second millennium BCE.
Of these, four of the five earliest livestock species, goats, sheep, pigs, and cattle, had wild ranges that overlapped with the cereal zone of the Fertile Crescent. This geographic coincidence is the single most important fact in early human history.
Nowhere else did humans have simultaneous access to multiple high-yield cereals and multiple large herbivores suitable for domestication. Eurasia’s other centers (China, India, the steppe) each lacked part of the combination: China had crops but few large mammals; India had animals but weaker cereals; Africa had herding but scarce storable grains; the Americas had rich crops but no beasts of burden. The Fertile Crescent alone possessed both.
The concentration of opportunity
When these overlapping species were domesticated, they created self-reinforcing synergies. Cattle and goats provided manure that restored soil fertility to fields of wheat and barley. Sheep produced fiber for textiles, encouraging trade. Pigs turned food waste into meat. Donkeys and oxen pulled carts that carried surplus grain to market. Each success magnified the productivity of the others. Within only a few thousand years, this cluster of species turned a single region’s ecology into a prototype of civilization.
Genetically, this zone also displayed extraordinary plasticity. The cereals of the Fertile Crescent were polyploid hybrids with flexible genomes; the ruminants that grazed its hills were social, hierarchical, and behaviorally tractable. The combination of genetic malleability and ecological compatibility explains why the first horticultural societies became agrarian so rapidly. Geography, through its intersection of wild ranges, created a biological “critical mass” that no other continent could easily replicate.
From this nucleus, agriculture spread outward in a great diffusion arc to Egypt, Anatolia, the Balkans, and eventually across Europe. The crops and animals of the Fertile Crescent carried with them not only calories but entire ecological relationships: seed to soil, manure to field, herd to pasture. As they moved, they adapted to new climates but retained their shared ancestry. Every loaf of bread, every glass of milk, every plowed field in medieval Europe ultimately traced its lineage back to those first species whose wild ranges overlapped in the highlands of the ancient Near East.
Genetic Foundations of Domesticated Animals
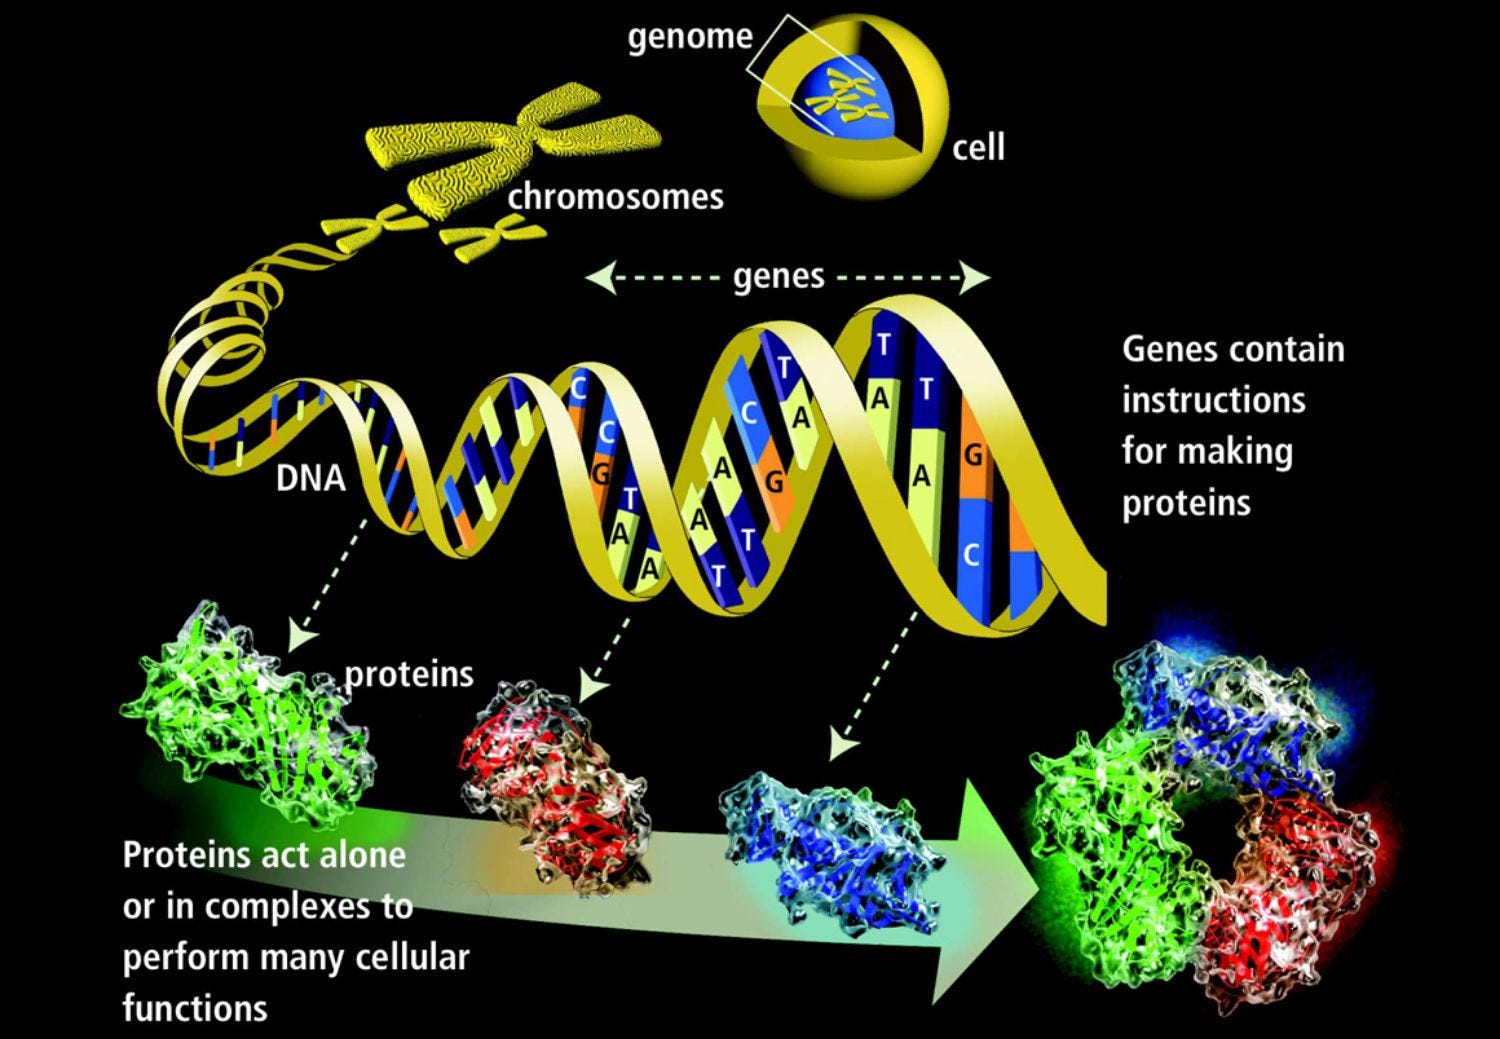
The genetic basis of domestication, once invisible to early herders, is now becoming clear through modern molecular studies. Research on cattle, goats, pigs, sheep, and dogs shows that domestication required only a few alleles of large effect to reshape entire behavioral and physical systems. These genes affected stress response, hormonal regulation, and social bonding: traits that together produced animals capable of cooperating with humans.
The key genetic changes
In cattle, for example, selection focused on genes such as MC1R and KIT, which affect coat color and indirectly signal reduced stress reactivity. In pigs, mutations in NR6A1 and IGF2 produced longer bodies and faster growth. Dogs show changes in genes associated with the hypothalamic–pituitary–adrenal (HPA) axis, notably WBSCR17, which modulates fear and sociability; this same locus is implicated in Williams syndrome in humans, a condition marked by hypersociability and low aggression. Goats and sheep exhibit selection in SLC35A5, STIM1, and other genes linked to tameness and adaptation to confinement.
Across species, these domestication genes cluster in pathways controlling neural crest cell development: the embryonic system that shapes pigmentation, facial structure, and parts of the nervous system. Slight reductions in neural crest activity yield the familiar domestication syndrome: floppy ears, shorter snouts, spotted coats, and calmer behavior. This genetic pattern explains why domestication produces similar physical changes in unrelated species. The same handful of developmental switches can be tuned to generate an animal both useful and docile.
The genetic evidence
Genome sequencing has confirmed that these changes arose rapidly under strong human selection. Most domesticated lineages show long regions of reduced genetic diversity, indicating powerful selective sweeps for key alleles. For example, dogs diverged from wolves less than 20,000 years ago yet display hundreds of fixed mutations in behavioral genes. Cattle and goats were domesticated around 8,000 BCE but already show deep genetic differentiation from their wild ancestors. In each case, the shift from fear to sociability was encoded by a few mutations that altered how the brain and hormones respond to stress.
These discoveries validate what early herders achieved intuitively. By favoring the most manageable animals, they unconsciously selected the same genes that modern science now identifies as the biological signature of domestication. The process reveals how easily behavior, physiology, and appearance can be rewired when the right genetic levers exist and how geography, by distributing those potential levers unevenly, constrained which societies could access animal power.
The biological threshold for cooperation
The domestication of animals thus depended on a biological threshold: a population had to contain individuals already predisposed to tameness, and humans had to encounter them frequently enough for selection to take hold. This combination occurred repeatedly in the Fertile Crescent, Central Asia, and East Asia, but rarely elsewhere. In sub-Saharan Africa and the Americas, the necessary behavioral variation was either absent or inaccessible. The result was not a failure of culture but a limitation of biology. Only where certain genes existed in wild populations could humans bring them under control.
Once this threshold was crossed, animal power reshaped the energy balance of human life. Every plow pulled by oxen, every field fertilized by manure, every wagon drawn by horses rested on a handful of mutations that softened fear, strengthened attachment, and allowed one species to cooperate with another. Those genetic accidents became the foundation for agrarian and, later, industrial civilization.
The First Great Unequal Endowment
The Fertile Crescent was not merely the birthplace of agriculture. It was the first region where geography and biology converged to make complex society possible. Its Mediterranean climate, alternating wet winters and dry summers, favored annual grasses and legumes. Its limestone hills and river valleys supported wild herds of sheep, goats, and cattle. Within a small area, early humans could gather high-calorie seeds, hunt large animals, and eventually combine the two into a single system of farming and herding. No other region offered such complementary resources so close together.
The result was a head start of several thousand years. Surpluses of grain and livestock supported permanent villages by 8000 BCE, cities by 4000 BCE, and empires soon afterward. The Fertile Crescent’s advantage was not cultural but ecological: its biodiversity created the conditions for innovation. When agriculture spread north and west into Europe, it carried the same species that had first evolved there. Wheat, barley, and cattle formed the basis of European agriculture for millennia. The Mediterranean climate belt effectively exported the Fertile Crescent’s biological endowment.
Yet geography remained a constraint. Regions far from this climatic corridor struggled to adapt its crops. The same wheat that thrived in Anatolia failed in the tropics; the same sheep that grazed the Levant could not survive in equatorial humidity. Agricultural diffusion slowed wherever climate or altitude broke continuity. In Diamond’s terms, Eurasia’s east–west axis allowed faster spread than Africa’s or the Americas’ north–south axes. But even within Eurasia, the biological limits of each species determined how far the revolution could go.
Agriculture: First Key to Progress
Agriculture did not create material progress, but it made progress possible. By producing a surplus of calories, early farmers freed part of the population from subsistence labor. That surplus could be stored, taxed, traded, or invested in new skills. Over time, it supported the rise of artisans, merchants, soldiers, and administrators, the first specialists in history. Horticultural and agrarian societies were therefore necessary steps in the evolution of more complex societies, even though they remained stagnant in living standards for millennia.
The transition from Horticultural to Agrarian societies depended heavily on the domestication of draft animals. The animal-driven plow was the first major labor-saving technology in history.
By multiplying the power of human muscle, it allowed larger fields to be cultivated and increased yields per worker. Regions that possessed cattle, horses, or water buffalo gained a decisive advantage in productivity. Those without them remained limited to hand tools and shifting cultivation. The biological availability of animal traction thus determined which societies could sustain dense populations and develop complex states.
Over the long run, this surplus created the conditions for Commercial societies. These societies invented four of the Five Keys to Progress. Regular exchange of surplus grain and animal products encouraged trade, markets, and money. The same roads that carried food also carried ideas and technologies. When Europe’s Commercial societies emerged in the late Middle Ages, they were building on an inheritance of agricultural productivity rooted in ancient domestication.
Only after the Industrial Revolution, however, did humans begin to transcend geography entirely. Fossil fuels replaced animal energy, fertilizers replaced manure, and mechanized transport replaced oxen and horses. But none of that would have been possible without the biological foundation laid ten thousand years earlier.
Animal Power
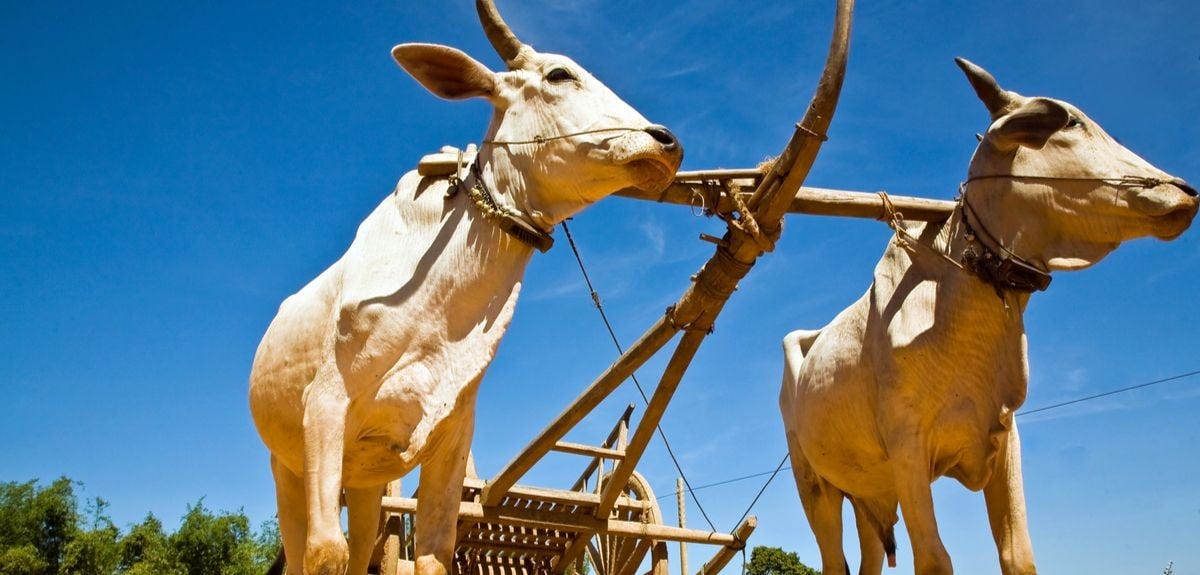
Animal traction was more than a tool. It was the first true energy revolution. By harnessing the strength of oxen, horses, and camels, humans increased their effective power output by orders of magnitude. A man could plow perhaps a tenth of a hectare per day; with oxen he could manage ten. This multiplication of labor enabled vast increases in arable land and allowed fewer farmers to feed more people. It also changed the structure of society: controlling draft animals became a form of capital, and those who owned them gained wealth and status.
The plow transformed landscapes as well as economies. It encouraged permanent fields, irrigation systems, and property rights. It linked rural villages to urban granaries through transport networks of carts and pack animals. In regions without large domesticable mammals, such as sub-Saharan Africa, the Americas, or Oceania, agriculture remained labor-intensive and less scalable. These societies could still achieve sophistication, but their material base was thinner. The global pattern of development for millennia reflected this biological disparity.
Commercial societies inherited and extended these advantages. By using animal power for transport and manufacturing, spinning wheels, mills, and pumps, they achieved levels of productivity unknown in purely agrarian systems. The animal was the prototype of the machine: a source of repeatable work independent of human fatigue.
When the British Industrial Revolution replaced animals with steam engines, it was merely substituting mechanical muscles for biological ones. The continuity between plow, mill, and engine is the continuity of energy substitution, each step building on the one before.

Diffusion of Agriculture to Europe
Once agriculture had arisen, its spread depended on the orientation and connectedness of the continents. Eurasia’s east–west axis allowed crops and animals to move thousands of kilometers with little change in day length or climate. Wheat and barley could grow from Mesopotamia to Spain; cattle could graze from Anatolia to the Rhine. This geographic continuity created a vast zone of compatible ecosystems where innovations diffused easily. The Americas and Africa, by contrast, were oriented north–south, crossing multiple climate zones that blocked diffusion. Maize from Mexico struggled in Andean altitudes; African sorghum faltered in Mediterranean climates.
These differences compounded over time. In Eurasia, the spread of agriculture supported dense populations and frequent interaction among states, generating competition and innovation. In Africa and the Americas, isolated centers of domestication remained regional. The Incas and Aztecs achieved remarkable organization, but their geographic fragmentation limited exchange. Geography thus constrained not only the origin but also the diffusion of progress. Even the most inventive societies could not easily transmit their breakthroughs across ecological barriers.
When European expansion began after 1500, these inherited asymmetries determined the outcome. The societies that had long benefited from wide diffusion and abundant domesticates descending from Commercial Europe industrialized first. Others followed according to the depth of their agrarian base. Geography had set the sequence centuries earlier.
The Long Legacy of Geography
The effects of early domestication extended far beyond agriculture. Over thousands of years, the interaction between humans, plants, and animals reshaped human biology itself. The ability to digest lactose, the spread of disease resistance, and even behavioral traits associated with settled life all evolved under the pressures of farming and herding. Human societies and genomes co-evolved with their domesticates.
This feedback produced large differences between populations exposed to long agricultural histories and those that were not. Agrarian peoples developed immunities to zoonotic diseases like smallpox and measles; hunter-gatherers did not. When Eurasian explorers reached the Americas, this biological imbalance proved catastrophic. The Columbian Exchange spread crops, animals, and pathogens worldwide, breaking the old geographic constraints for the first time but also revealing how deeply biology had shaped civilization’s map.
Over the very long term, these interactions even altered patterns of human selection. In settled societies, success depended less on raw physical strength and more on social and cognitive skills: planning, cooperation, and foresight. Individuals with these traits tended to achieve higher status and reproduce more. Over many generations, such selection may have shifted the distribution of heritable characteristics that support complex behavior. In this sense, the biogeography of domestication indirectly influenced human evolution itself.
Overcoming geographical constraints
The long chain of causation that began with geography and biology ultimately produced a world able to transcend them. The innovations of Commercial and Industrial societies, markets, science, and technology, transformed progress from a local accident into a global process.
Yet the sequence remained consistent: societies industrialized in roughly the same order as their ancestors achieved earlier stages of complexity. Those whose genetic and cultural lineages traced back to the Commercial and Free-Peasant societies of 1500 Europe, Britain, the Low Countries, northern Italy, and their offshoots, were first to industrialize. Societies descending from later Agrarian stages followed more slowly, and those rooted in Horticultural or Herding traditions lagged further still.
Industrial technology finally broke the old geographic constraints. Fossil fuels replaced the need for local domesticates; chemistry replaced the fertility of specific soils. For the first time, any region could achieve prosperity regardless of its biological inheritance. But the sequence of progress, the order in which societies rose, remained a record of ancient geography. The foundations of modern wealth were laid not in the nineteenth century but in the Neolithic fields of the Fertile Crescent.
Conclusion: From Geographical Constraints to Human Progress
The geography of wild ancestors set the stage for all of human history. It defined where agriculture could begin, where animals could be tamed, and where early surpluses could support the first complex societies. The Fertile Crescent, China, and a few other fortunate regions inherited plants and animals whose genomes happened to be open to domestication. From these biological starting points, horticultural and agrarian societies evolved. These society types laid the demographic and institutional groundwork for later Commercial and Industrial civilization.
Yet these early transformations did not themselves create material progress. For thousands of years, most people lived near subsistence despite rising complexity. Progress required something more: the accumulation of knowledge, competition, and freedom within networks large enough to sustain continuous innovation. That leap occurred only in the Commercial societies of early modern Europe, descendants of regions long shaped by agriculture, trade, and animal power. When those societies finally harnessed fossil fuels during the Industrial Revolution, they broke free from the constraints that had governed all previous eras.
In the language of The Five Keys to Progress, geography and biology provided the first preconditions, the resources and incentives, but not the mechanisms of progress itself. The later rise of decentralized exchange, open competition, and technological adaptation completed the sequence.
Nature determined where humanity could begin the climb; culture determined how high it could go. The pattern of global development since 1500 reflects this layered inheritance: nations industrialized in the same order that their ancestors evolved more complex societies, because complexity itself had become a biological and institutional legacy.
The great achievement of modern civilization, beginning in Britain and spreading outward, was to transcend these natural limits. Industrial technology replaced the luck of geography with the universality of human problem-solving. The wild ancestors of wheat, barley, and cattle no longer defined destiny; the keys to progress had shifted from the soil to the mind. Humanity’s greatest triumph, after ten thousand years of constraint, was to turn the inheritance of geography into a platform for freedom.
Bibliography
If you are interested in reading more on this topic, I would recommend:
Diamond, Jared. Guns, Germs, and Steel: The Fates of Human Societies. W. W. Norton, 1997.
Vavilov, Nikolai I. Origin and Geography of Cultivated Plants. Cambridge University Press, 1992 (posthumous translation).
Murphy, Denis J. People, Plants, and Genes: The Story of Crops and Humanity. Oxford University Press, 2007.
Zeder, Melinda A. Feeding the World: Archaeology and the Agricultural Revolutions. University of California Press, 2011.
Scott, James C. Against the Grain: A Deep History of the Earliest States. Yale University Press, 2017.
Mazoyer, Marcel, and Laurence Roudart. A History of World Agriculture: From the Neolithic Age to the Current Crisis. Monthly Review Press, 2006.
Smil, Vaclav. Energy and Civilization: A History. MIT Press, 2017.
Technical Bibliography
The section on specific genetic alleles that enable the domestication of wild ancestors is based on:
Allaby, Robin G., et al. “Domestication as Innovation: The Genomic Foundations of Agricultural Enhancement.” Proceedings of the National Academy of Sciences 116, no. 25 (2019): 12245–12252.
Larson, Greger, and Dorian Q. Fuller. “The Evolution of Animal Domestication.” Annual Review of Ecology, Evolution, and Systematics 45 (2014): 115–136.
Purugganan, Michael D., and Dorian Q. Fuller. “The Nature of Selection during Plant Domestication.” Nature 457, no. 7231 (2009): 843–848.
Freedman, Adam H., et al. “Genome Sequencing Highlights the Dynamic Early History of Dogs.” PLoS Genetics 10, no. 1 (2014): e1004016.
Belyaev, Dmitry K. “Destabilizing Selection as a Factor in Domestication.” Journal of Heredity 70, no. 5 (1979): 301–308.
Gross, Benjamin L., and Kenneth M. Olsen. “Genetic Perspectives on Crop Domestication.” Trends in Plant Science 15, no. 9 (2010): 529–537.
Meadows, Jennifer R. S., et al. “Globally Distributed Single-Origin Domestication of the Goat.” Proceedings of the National Academy of Sciences 108, no. 1 (2011): 1–6.
If you enjoyed this article, you should read my From Poverty to Progress book series.
Interesting correlations. I suppose our predisposition to sociality had to precede the discovery of compatible plants and animals for domestication, so we could discuss, plan, and organize the necessary collection, harvesting, irrigation practices, etc.
On loss of plant dormancy, I had to delve into Wiki to understand this, which says: "Dormant seeds do not germinate in a specified period of time under a combination of environmental factors that are normally conducive to the germination of non-dormant seeds. An important function of seed dormancy is delayed germination, which allows dispersal and prevents simultaneous germination of all seeds." If I now understand this criterion for aiding domestication correctly, this meant most of the seeds collected and planted would grow over the same general season and thus aid cooperation to harvest and store the result, providing a concentrated output in a relatively short time. In contrast, seeds without this characteristic would have their germination and growth cycles spread out over a more extended time span that would not be as conducive for joint social activity, or net quantitative output.
So what worked well for evolution to support the existence of some sort of grass specie had to be selected against to aid domestication of the more human helpful varieties.
On animal domestication by finding species compatible with human presence and reduced levels of aggression or flight, I still wonder that even after many thousands of years of failing to find such features in some species (say zebras) that a program of selection plus genetic "interference" or gene "therapy" might lead to a more domestically friendly variety. But today, for example, horses can provide what zebras might have been bred to do. But are there species, such as perhaps fur bearing ones, that might still be of value to humanity to develop domesticated versions?* Dolphins are not exactly domesticated but can be trained to aid in maritime exploits of a military nature (and entertainment and maybe others?). Maybe seals or penguins could be trained to provide fish for humans? Just spit balling here. :-)
*Just had the thought that I suppose development of micro-organisms that can "eat" oil spills or help reduce pollution would also qualify - we don't necessarily need mammal sized contributors.